Timing and Reward in Perceptual Decision-Making

Post by Cody Walters 

What’s the science?

Decision-making often takes place in dynamic and uncertain environments, yet it remains poorly understood how this uncertainty affects time-sensitive decision-making strategies. This week in The Journal of Neuroscience, Shinn and colleagues, used a novel model to identify the cognitive mechanisms that explain behaviour during a perceptual decision-making task under temporally uncertain conditions.

How did they do it?

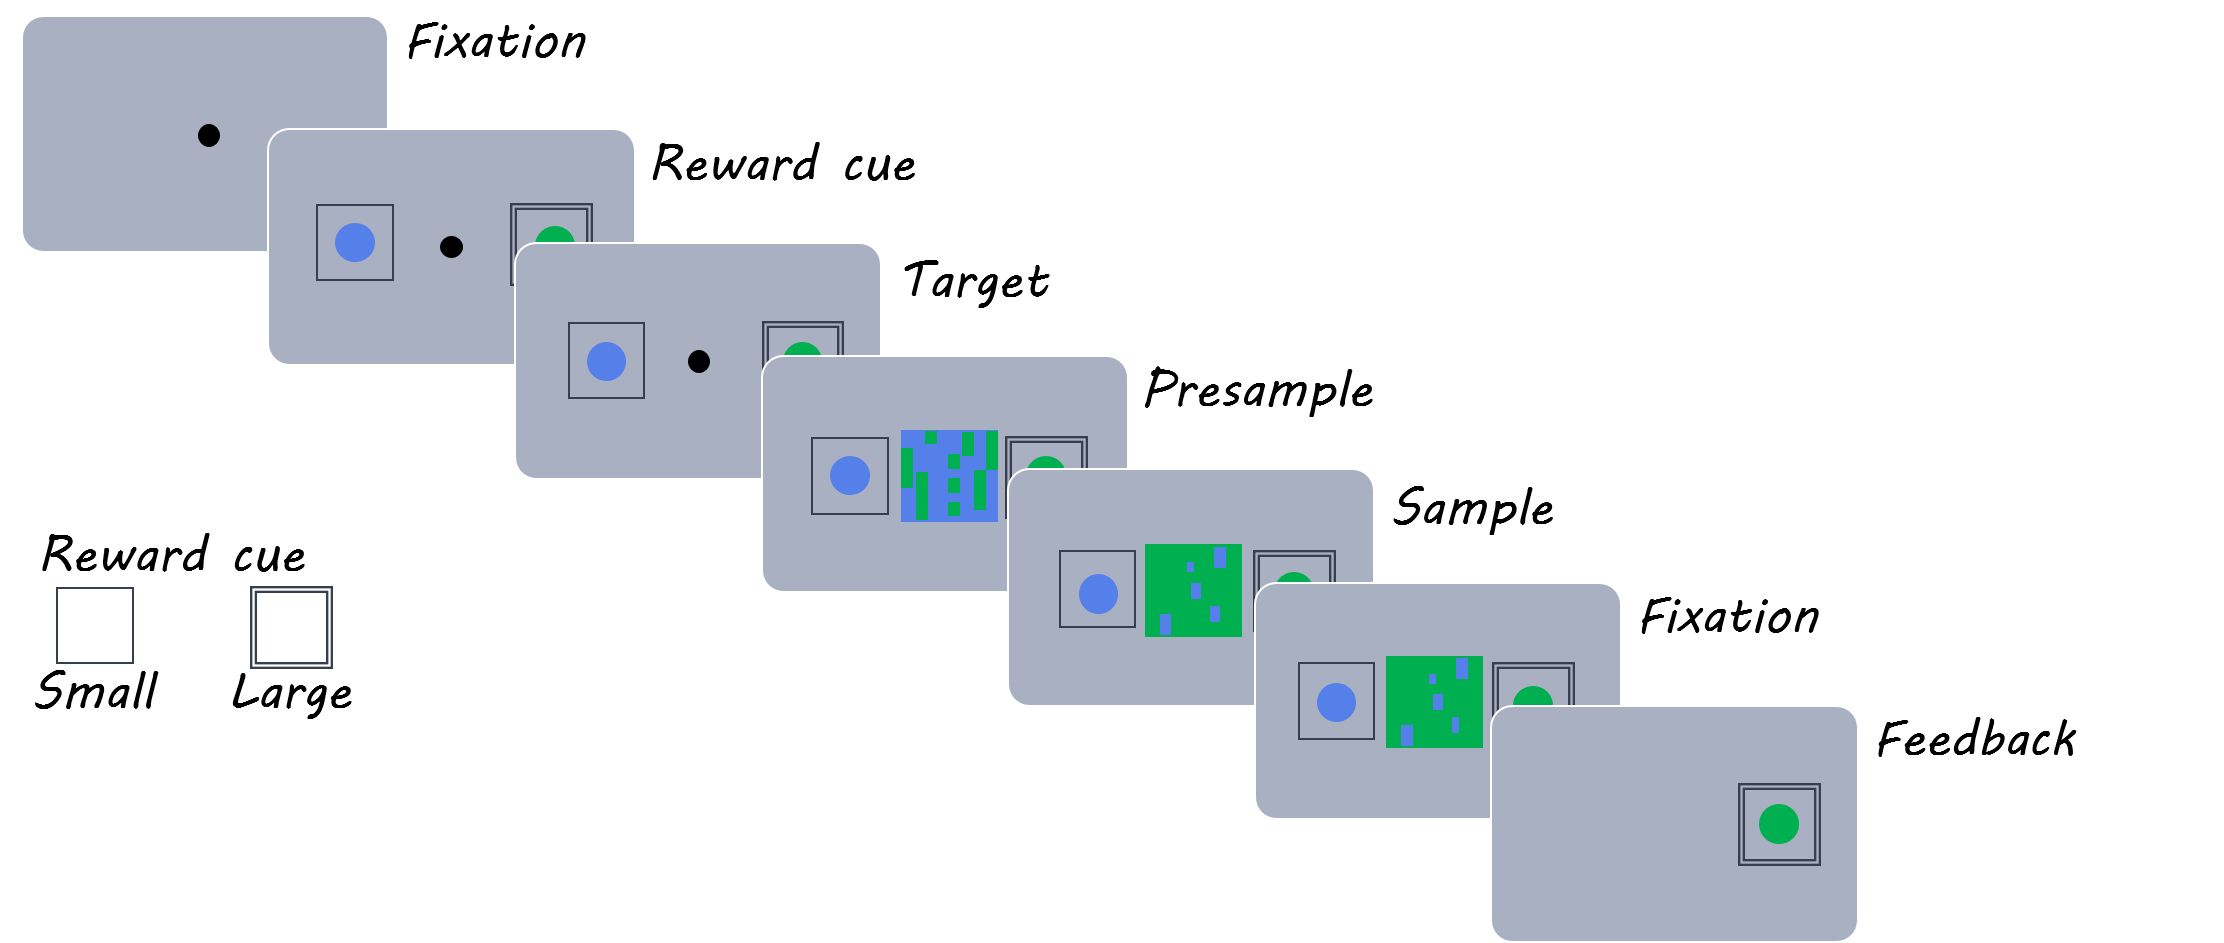
The authors trained two male rhesus macaques (monkeys) to perform a color-matching task. The animals fixated on a screen and were presented with a square grid (i.e., the ‘sample’) of randomly arranged blue and green pixels. The animals then had to indicate whether there were more blue or green pixels in the image by saccading (i.e., moving their eyes) to the corresponding color-coded target on the left or right of the sample in order to receive a juice reward. While the animals fixated on the screen prior to the sample being displayed, the targets indicated which of the two colors, if correctly selected, would result in a larger reward for that trial. Additionally, there was a non-informative ‘presample’ grid of blue and green pixels that was displayed for either 400 or 800 milliseconds preceding the onset of the sample.
cody (3).png

To model evidence accumulation, the authors used drift-diffusion models (DDMs). A DDM captures how perceptual information is integrated over time and ultimately results in a choice being made between one of two alternatives. DDMs fundamentally involve a drift rate (how quickly the decision variable is accumulated) and decision boundary (which, when reached, triggers a response). In addition to a traditional DDM, the authors also used an extended version that they refer to as a generalized drift-diffusion model (GDDM). A GDDM incorporates features such as time-varying evidence accumulation (a ‘leak’ parameter), an urgency signal to discourage prolonged deliberation (through either a ‘collapsing bounds’ or ‘linear gain’ parameter), and reward bias (through either an ‘initial bias’ parameter that shifts the starting point of the decision variable, a ‘time-dependent bias’ parameter that accelerates the decision variable toward the direction of the larger reward option, or a ‘mapping error’ parameter that accounts for movement errors). Furthermore, a delay parameter was introduced to the urgency signals to model the uncertainty surrounding the stimulus onset.

What did they find?

The authors compared two DDM models in order to determine which provided a better fit to the monkeys’ choice and reaction time data. They found that the GDDM, relative to a reward-biased DDM (a traditional DDM with initial bias and time-dependent bias parameters), more accurately captured the choice and reaction time data and provided a better fit to the errors resulting from reward bias (where the monkeys would choose the large-reward option when the evidence favored the small-reward option). These findings suggested that the GDDM was needed in order to more closely examine the mechanisms influencing evidence accumulation under conditions of temporal uncertainty.

The authors then fit multiple GDDMs (with different parameter combinations) to the choice and reaction time data obtained from the two monkeys. They found that models with time-varying urgency outperformed models with a constant urgency signal (such as the traditional DDM), suggesting that whatever strategy the animals used to adapt to the temporal uncertainty of the stimulus onset was being captured by the time-varying urgency parameter. As for reward parameters, they found that a combination of initial bias (an integration-dependent mechanism) with mapping error (an integration-independent mechanism) provided the best fit to the experimental data. To address the extent to which the leak parameter and the time-varying urgency signal functionally overlapped, the authors then removed the leak parameter from the GDDMs. They found that GDDMs with a time-varying urgency parameter but without a leak parameter experienced significant impairment in performance, thus suggesting that leaky evidence accumulation improves the model fits by discounting earlier, more uncertain sensory evidence through a separate mechanism from the time-varying urgency signal.

Next, the authors investigated whether within-session changes in the temporal context would influence the urgency signal using a modified version of the task. Importantly, this task design ensured that 20% of trials in both the short and long presample blocks had a 0.75 second presample, which allowed the authors to assess the extent to which temporal context affected the urgency signal. The authors found that the best-fit GDDM obtained from the first task fit the monkey data from the modified task exceptionally well, with the urgency parameter alone accounting for most of the variation in the data. These findings show that the monkeys’ behavioral strategy in different temporal contexts is explained in large part by the timing of the urgency signal. Finally, the authors showed that modulation of the urgency signal (i.e., the decision boundary collapse delay) alone is sufficient to influence a speed-accuracy tradeoff, thus demonstrating an overall role for the urgency signal in time-dependent decision-making strategies.  

What’s the impact?

These findings demonstrate that (1) a dynamic urgency signal provides a flexible mechanism for incorporating sensory evidence into the decision-making process under temporal uncertainty and (2) that integration-dependent (initial bias and time-dependent bias) and integration-independent (mapping error) mechanisms are both required to explain reward bias. Overall, these data suggest that time is an important factor affecting how subjects integrate information and make decisions. Further, this study outlines a promising new model for exploring the cognitive mechanisms underlying perceptual decision-making.
decision_quote_sep1.jpg

Confluence of timing and reward biases in perceptual decision-making dynamics. The Journal of Neuroscience (2020). Access the original scientific publication here.
Modes of Adolescent Brain Development

Post by Anastasia Sares 

What's the science?

During adolescence, the brain is developing in leaps and bounds, a process we still don’t fully understand. There are many factors that can have competing influences on the growing brain, like physical health, financial situation, or social ties. Since 2016, one large longitudinal study (the “Adolescent Brain and Cognitive Development” or ABCD study) has focused on tracking data related to adolescent brain development in almost 10,000 individuals. This week in Biological Psychiatry, Modabbernia and colleagues delved into this large dataset in order to find patterns of interaction in adolescent brain development involving many brain-based, behavioural, and environmental factors all at once, rather than focusing on one or two in isolation. 

How did they do it?

The authors used a technique called Canonical Correlation Analysis (CCA) to discover relationships between sets of life factors and sets of brain outcomes. Some examples of the life factors measured included: mother’s age and health at birth, childhood medical conditions, height and weight, sleep quality, intelligence scores, prosocial behavior, number of friends, screen time, family finances, neighborhood air quality, and local crime statistics. Examples of the brain outcomes included: brain volume, thickness and surface area of the cortex (the brain’s outer layer), integrity of the white matter (internal connections between different brain areas), and brain activity at rest. Each of the brain measures were taken for multiple brain regions. The authors used 85% of the data to form a model describing these relationships, and then used the leftover 15% of the data to test the model and see if the relationships held. 

What did they find?

The results yielded 14 different “modes,” or patterns of brain/behaviour/environment covariation. Many of the modes showed the kinds of relationships we’d expect: for example, teens with better physical health and a richer social and cognitive environment had larger brain volumes and more brain surface area. They also had better connectivity between their prefrontal cortex and other brain regions. There were also some more specific, less standard patterns. For example, a combination of high academic ability and socioeconomic status with abnormal sleep and mood was associated with a thinning of the cortex. This may be the trajectory followed by people who later develop bipolar disorder. The authors also noted that “positive and negative exposures do not occur in isolation but cluster together” and that basic characteristics like height and weight can have a huge effect on measures of brain structure. These are important considerations for future studies to take into account.

What's the impact?

This work confirms a lot of connections made by previous research, identifying consistent patterns of brain, behavioural and environmental factors in a large sample of adolescents. It also suggests key clusters of variables that could be targets for intervention in adolescent development.

Modabbernia et al. Multivariate Patterns of Brain-Behavior-Environment Associations in the Adolescent Brain and Cognitive Development (ABCD) Study. Biological Psychiatry (2020). Access the original scientific publication here.

Uncovering Proteins That Interact with a Disease Form of Tau

Post by D. Chloe Chung

What's the science?

Tau is a microtubule-binding protein that normally contributes to the stability of the central nervous system. In multiple neurodegenerative diseases including Alzheimer’s disease, tau becomes abnormally phosphorylated and detaches from microtubules, leading to synaptic dysfunctions and neuronal death. Many studies have investigated the exact mechanisms of how tau phosphorylation contributes to the disease course, but there is a gap in knowledge of what types of proteins interact with phosphorylated tau (pTau). This week in Brain, Drummond, Pires, and colleagues use complementary proteomics approaches to discover previously unknown protein interactors of pTau.

How did they do it?

Neurofibrillary tangles (NFTs), composed of pTau, were dissected and isolated from brain samples of Alzheimer’s disease patients using a laser-capture microdissection technique. These samples were analyzed to identify proteins other than pTau that are present in NFTs. pTau was extracted along with its protein interactors from the Alzheimer’s disease brain tissue. Here, an antibody that can detect a specific phosphorylation site on tau was used to isolate the pTau-interactor complex. Using these samples, the profile of pTau and its interacting proteins was compared to the list of NFT-associated proteins. Also, pTau-interacting proteins were categorized based on related biological pathways or protein families to better understand which biological aspects are closely related to pTau.

What did they find?

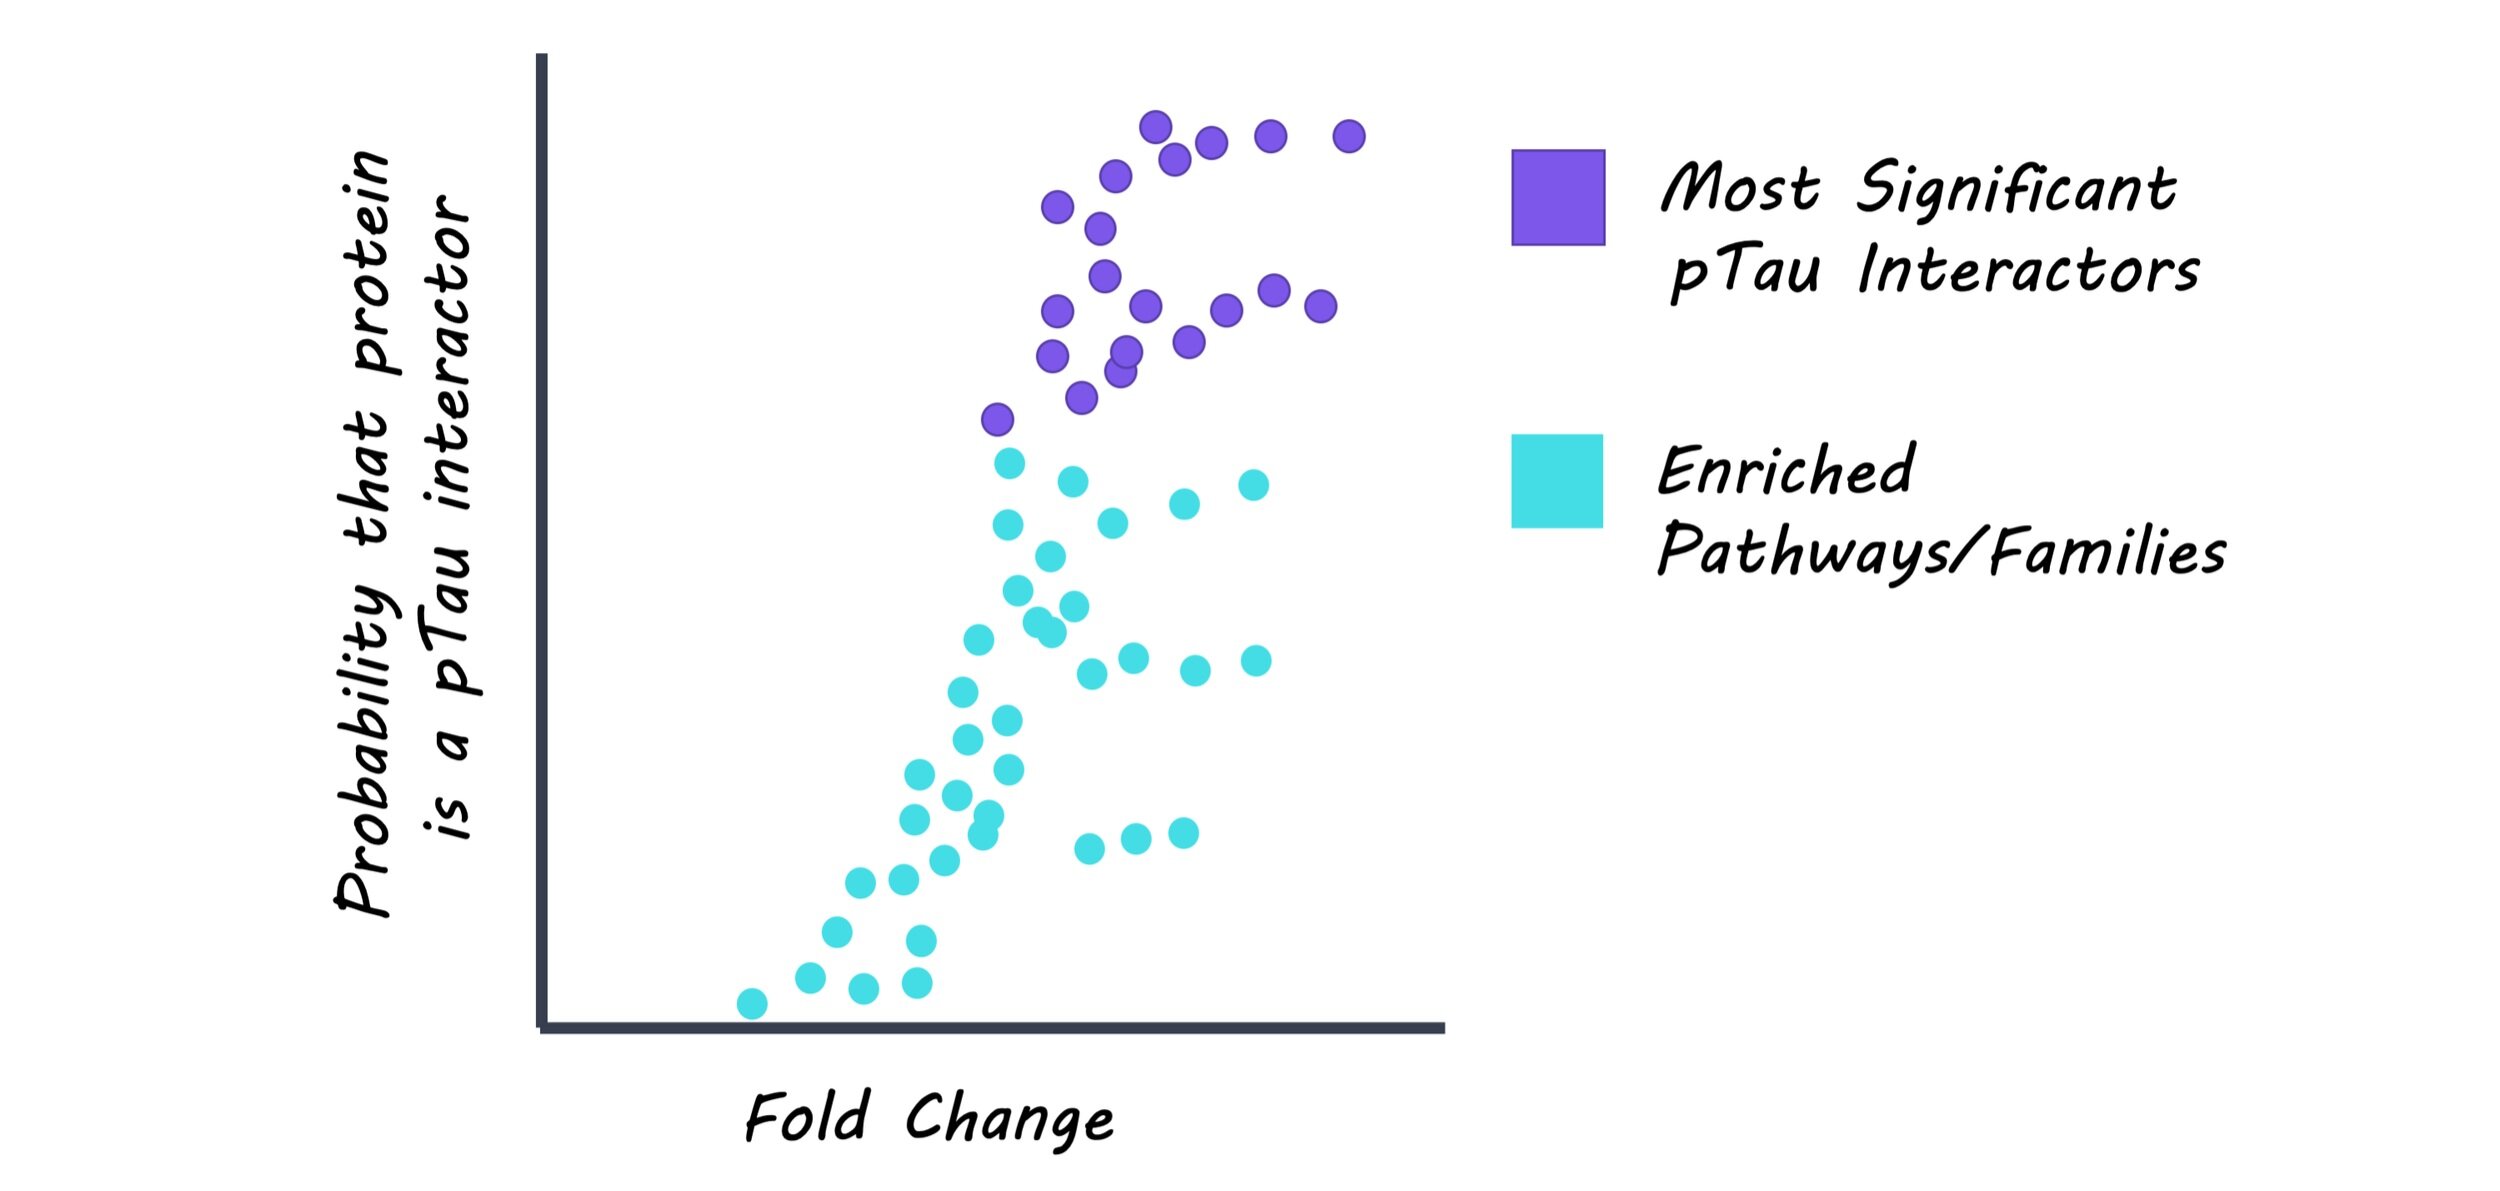
From the first proteomics analysis, the authors found 542 proteins to be present in NFTs, including tau and other proteins that have been well-documented for their association with NFTs. From the second proteomics analysis, the authors found 125 proteins that interact with pTau. Interestingly, many of pTau interactors were associated with two major protein degradation pathways: one involved ubiquitin that tags proteins to be degraded by proteasomes, and the other involved lysosomes that break down proteins with digestive enzymes. These findings suggest an important pathological link between pTau and impaired protein degradation, which has been largely hypothesized in the field. Importantly, the authors compared two proteomics datasets and found that 75 out of 125 pTau-interacting proteins were also present in NFTs. Among them, 12 proteins have never been reported to interact with pTau before, meaning that the authors found new pTau-interacting proteins from their analysis. The type of these new pTau interactors varied, ranging from proteins that bind to DNA or RNA to subunits of enzymes or ribosomes.

tau_image_aug25.jpg

What’s the impact?

While there have been several studies that have reported protein interactors of tau, this study is the first to find proteins that interact specifically with phosphorylated Tau in the human brain. In particular, this work identified novel proteins that have never been reported to be associated with tau before, opening new areas to investigate tau biology. Findings from this study will elevate our understanding of how tau exerts its toxic effects in the brain upon phosphorylation. Also, this study will be useful in identifying potential drug targets to treat Alzheimer’s disease and other neurodegenerative diseases in which tau is abnormally phosphorylated.

Brain_quote_Aug24.jpg

Drummond, Pires et al. Phosphorylated tau interactome in the human Alzheimer’s disease brain. Brain (2020). Access the original scientific publication here.